 Coach
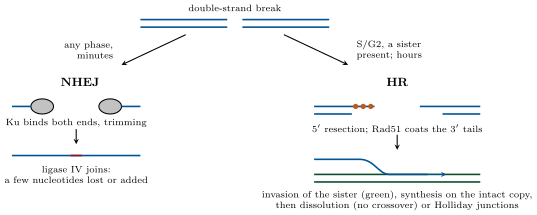
A double-strand break severs the chromosome and has no intact strand to copy. Two pathways repair it. Non-homologous end joining (NHEJ): the Ku70–Ku80 ring binds each end, recruits the kinase DNA-PKcs, nucleases trim overhangs, and ligase IV joins the ends; it works at any stage of the cycle and in minutes, but loses or adds a few nucleotides at the junction and can join the wrong ends. Homologous recombination (HR): the MRN complex and nucleases resect the 5 strands to leave long 3 single-stranded tails, which are coated by RPA and then, with the help of BRCA2, by the recombinase Rad51; the Rad51 filament searches for a homologous duplex — the sister chromatid, in S and G2 — invades it, and the invading 3 end primes synthesis on the intact copy. The joint molecules may be dissolved after a short synthesis (most mitotic repair, no exchange of flanking DNA) or mature into two four-way Holliday junctions, whose resolution by endonucleases yields either a crossover or a non-crossover product. HR is accurate because it copies a sister, but is available only when a sister exists.
示例
Example 3.9 (Why xeroderma is a disease of the fork)
A dose of sun leaves pyrimidine dimers in a keratinocyte. With a nucleotide excision half-life of () and a fork arriving after , dimers are still there to be copied; with the near-absent repair of an XP cell (), are. Each dimer met by the fork is bypassed by translesion synthesis (below), which is error-prone: the patient’s mutation load per division is fifteen times the normal one, and the skin cancers follow in childhood. The cure that works is to keep small — total avoidance of ultraviolet light.
Example 3.13 (Synthetic lethality: BRCA and PARP)
Women who inherit one defective copy of BRCA1 or BRCA2 have a lifetime risk of breast cancer of ; the tumours arise in cells that have lost the second copy and can no longer do homologous recombination. Such cells repair their double-strand breaks by end joining alone and accumulate rearrangements. They also acquire a specific weakness. Single-strand breaks, some a day, are repaired by a route that needs the enzyme PARP; when PARP is inhibited by a drug, single-strand breaks persist to S phase, where a fork converts each into a double-strand break with only one end — repairable only by recombination. A normal cell, with one good BRCA allele, copes; the tumour cell dies. Two defects, each harmless alone, are lethal together: the drug kills by synthetic lethality, and spares the patient’s other cells.